CH. 34 Nucleotide Syn 3
Study these flashcardsFree · spaced repetition · iPhone, Android, Mac & web
All cards
1
The pyrimidines are , , and
The pyrimidines are cytosine, uracil, and thymine
2
The first step of pyrimidine biosynthesis involves the formation of de novo synthesis of a pyrimidine
The first step of pyrimidine biosynthesis involves the formation of carbamoyl phosphate de novo synthesis of a pyrimidine
3
The formation of the caramoyl phosphate requires , , and [derived from hydrolysis].
The formation of the caramoyl phosphate requires 2 ATP, Bicarbonate (HCO3-), and Ammonia (NH3) [derived from glutamine hydrolysis].
4
CPS II is allosterically regulated in 2 ways:
• Activated by , , and
• Inhibited by ,
• Activated by , , and
• Inhibited by ,
CPS II is allosterically regulated in 2 ways:
• Activated by PRPP, ATP (purine -> for balance), and glutamine
• Inhibited by UDP, UTP (end-products)
• Activated by PRPP, ATP (purine -> for balance), and glutamine
• Inhibited by UDP, UTP (end-products)
5
The second step of pyrimidine synthesis requires carbamoyl conversion to
The second step of pyrimidine synthesis requires carbamoyl conversion to orotate
6
In the conversion of carbamoyl to orotate, joins through to make
• After a couple of reactions makes -> , which has the basic pyrimidine ring shape.
• After a couple of reactions makes -> , which has the basic pyrimidine ring shape.
In the conversion of carbamoyl to orotate, Asp joins through aspartate transcarbamoylase (ATCase) to make carbamoyl aspartate
• After a couple of reactions Dihydroorotase makes -> Orotate, which has the basic pyrimidine ring shape.
• After a couple of reactions Dihydroorotase makes -> Orotate, which has the basic pyrimidine ring shape.
7
In the third step of pyrimidine synthesis, orotate is combined with to form
In the third step of pyrimidine synthesis, orotate is combined with PRPP to form OMP
8
After synthesis of orotate, the ring joins via the enzyme orotate phosphoribosyl transferase to form
After synthesis of orotate, the ring joins PRPP via the enzyme orotate phosphoribosyl transferase to form OMP
9
The fourth step of pyrimidine biosynthesis involves the formation of a base. Orotidylate (OMP) is decarboxylated via to form .
The fourth step of pyrimidine biosynthesis involves the formation of a uracil base. Orotidylate (OMP) is decarboxylated via orotidylate decarboxylase (UMP synthase) to form UMP.
10
UMP is converted to UTP using
UMP is converted to UTP using 2 ATP
11
What enzyme adds the P's to UMP?
The first - added by
The second - added by
The first - added by
The second - added by
What enzyme adds the P's to UMP?
The first - added by UMP kinase
The second - added by NDKP
The first - added by UMP kinase
The second - added by NDKP
12
*** TQ
UTP then gets converted to by , which uses and .
UTP then gets converted to by , which uses and .
*** TQ
UTP then gets converted to CTP by cytidylate synthetase, which uses glutamine and ATP.
UTP then gets converted to CTP by cytidylate synthetase, which uses glutamine and ATP.
13
is the only nucleotide synthesized de novo directly as a , since it arises directly from UTP.
CTP is the only nucleotide synthesized de novo directly as a triphosphate, since it arises directly from UTP.
14
CTP is useful for RNA synthesis. In order to become , it must first be dephosphorylated.
• An enzyme that does that is .
• An enzyme that does that is .
CTP is useful for RNA synthesis. In order to become dCTP, it must first be dephosphorylated.
• An enzyme that does that is apyrase: CTP -> CDP.
• An enzyme that does that is apyrase: CTP -> CDP.
15
***TQ
Order of synthesis of pyrimidines:
Order of synthesis of pyrimidines:
***TQ
Order of synthesis of pyrimidines: U -> C -> T
Order of synthesis of pyrimidines: U -> C -> T
16
dUTP is useless for synthesis. It should not be incorporated into . dUTP is a problem for the cell if DNA polymerase
recognizes dUTP just like and it will put dUTP into
DNA if it finds it!
recognizes dUTP just like and it will put dUTP into
DNA if it finds it!
dUTP is useless for RNA synthesis. It should not be incorporated into DNA. dUTP is a problem for the cell if DNA polymerase
recognizes dUTP just like dTTP and it will put dUTP into
DNA if it finds it!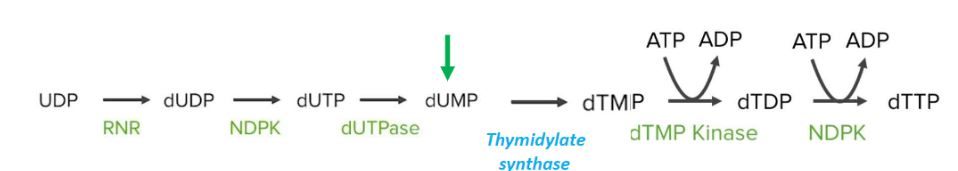
recognizes dUTP just like dTTP and it will put dUTP into
DNA if it finds it!
17
dUTP quickly gets converted into dUMP via
dUTP quickly gets converted into dUMP via dUTPase 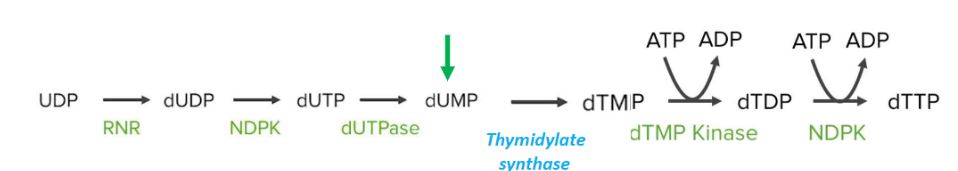
18
makes dTDP
dTMP kinase makes dTDP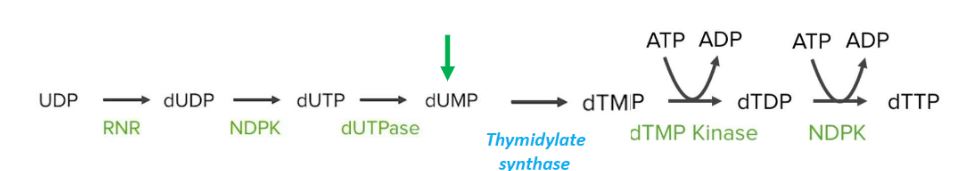
19
makes dTDP
dTMP kinase makes dTDP
20
makes dTTP.
NDPK makes dTTP.
21
is not regulated. If it finds a NDP or a dNDP, it will turn it into NTP or dNTP.
NDPK is not regulated. If it finds a NDP or a dNDP, it will turn it into NTP or dNTP.
22
If is not functional,you can’t replicate DNA! ( ->
If thymidylate synthase is not functional,you can’t replicate DNA! (dUMP -> dTMP)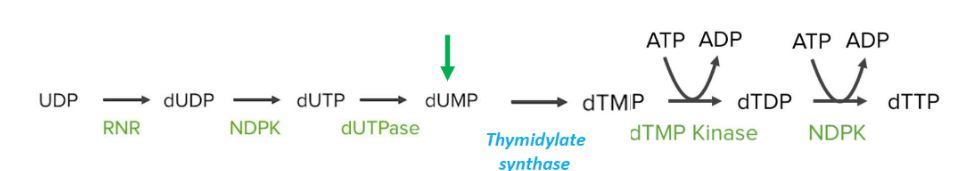
23
dUTP can also be directly made from deamination of
dUTP can also be directly made from deamination of dCTP 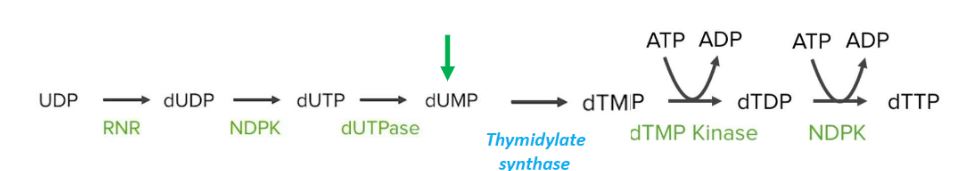
24
C1 unit can be used directly as in the conversion of to by Thymidylate Synthase
C1 unit can be used directly as N5-N10-methylene-THF in the conversion of dUMP to dTMP by Thymidylate Synthase 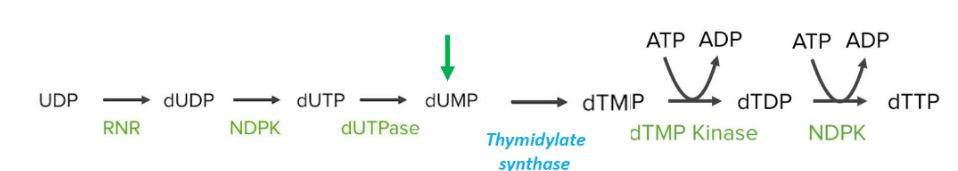
25
THF is to dihydrofolate in
this reaction.
(Anti-metabolites rxn)
this reaction.
(Anti-metabolites rxn)
THF is oxidized to dihydrofolate in
this reaction.
(Anti-metabolites rxn)
this reaction.
(Anti-metabolites rxn)
26
FH2
is reduced to FH4 by
. This is
called recycling.
is reduced to FH4 by
. This is
called recycling.
FH2
is reduced to FH4 by
dihydrofolate reductase. This is
called folate recycling.
is reduced to FH4 by
dihydrofolate reductase. This is
called folate recycling.
27
TEST QUESTION
-When THF recovery is blocked ( is not happening) with , the DHF reductase binds to with . It causes the indirect blockage of
-When THF recovery is blocked ( is not happening) with , the DHF reductase binds to with . It causes the indirect blockage of
TEST QUESTION
-When THF recovery is blocked (folate recycling is not happening) with MTX, the DHF reductase binds to MTX with greater affinity. It causes the indirect blockage of DNA synthesis.
-When THF recovery is blocked (folate recycling is not happening) with MTX, the DHF reductase binds to MTX with greater affinity. It causes the indirect blockage of DNA synthesis.
28
, a pro-drug, gets converted to . It Covalently binds and permanently Inhibits This process specificially blocks synthesis and synthesis.
5-Flurouracil, a pro-drug, gets converted to FdUMP . It Covalently binds and permanently Inhibits thymidylate synthase. This process specificially blocks DNA synthesis and dTMP synthesis.
29
dysfunction, as well as and/or deficiencies result in
decreased DNA synthesis
• causes megaloblastic anemia
decreased DNA synthesis
• causes megaloblastic anemia
Thymidylate synthase dysfunction, as well as Folate (vitamin
B9) and/or cobalamin (vitamin B12) deficiencies result in
decreased DNA synthesis
• causes megaloblastic anemia
B9) and/or cobalamin (vitamin B12) deficiencies result in
decreased DNA synthesis
• causes megaloblastic anemia
30
If vitamin B12, which accepts methyl groups from 5-methylTHF, is deficient, accumulates.
If vitamin B12, which accepts methyl groups from 5-methylTHF, is deficient, 5-methyl-THF accumulates.
31
Remember that 5-Me-THF is needed for synthesis of
from .
from .
Remember that 5-Me-THF is needed for synthesis of
methionine from homocysteine.
methionine from homocysteine.
32
Since 5-methyl-THF cannot be reconverted to otherfolate
derivatives, a deficiency is secondarily produced (the
methyl trap theory).
derivatives, a deficiency is secondarily produced (the
methyl trap theory).
Since 5-methyl-THF cannot be reconverted to otherfolate
derivatives, a folate deficiency is secondarily produced (the
methyl trap theory).
derivatives, a folate deficiency is secondarily produced (the
methyl trap theory).
33
Pyrimidine rings can be degraded to
and , which can then be excreted
via the lungs and kidneys.
and , which can then be excreted
via the lungs and kidneys.
Pyrimidine rings can be degraded to CO2
and ammonia, which can then be excreted
via the lungs and kidneys.
and ammonia, which can then be excreted
via the lungs and kidneys.
34
UTP and CTP can get hydrolyzed via , yielding and
UTP and CTP can get hydrolyzed via apyrase, yielding UMP and CMP
35
The 1st step in pyrimidine nucleotide degradation from and is to the nucleosides by pyrimidine-specific 5’-nucleotidases, yielding and .
The 1st step in pyrimidine nucleotide degradation from UMP and CMP is dephosphorylation to the nucleosides by pyrimidine-specific 5’-nucleotidases, yielding cytidine and uridine.
36
A is a hydrolytic enzyme that catalyzes the hydrolysis of nucleoside monophosphate into
nucleoside and phosphate.
nucleoside and phosphate.
A nucleotidase is a hydrolytic enzyme that catalyzes the hydrolysis of nucleoside monophosphate into
nucleoside and phosphate.
nucleoside and phosphate.
37
Cytidine and uridine are broken-down by into sugar-P + pyrimidine.
• use Pi (instead of water) to phosphorylase the pyrimidine from the (deoxy)ribose, yielding .
• use Pi (instead of water) to phosphorylase the pyrimidine from the (deoxy)ribose, yielding .
Cytidine and uridine are broken-down by pyrimidine phosphorylase into sugar-P + pyrimidine.
• nucleoside phosphorylases use Pi (instead of water) to phosphorylase the pyrimidine from the (deoxy)ribose, yielding sugar-P.
• nucleoside phosphorylases use Pi (instead of water) to phosphorylase the pyrimidine from the (deoxy)ribose, yielding sugar-P.
38
The final break-down molecule of both cytosine and uracil is
The final break-down molecule of both cytosine and uracil is acetyl CoA
39
The break-down to thymine yields
which can go into TCA cycle.
which can go into TCA cycle.
The break-down to thymine yields
succinyl CoA which can go into TCA cycle.
succinyl CoA which can go into TCA cycle.
40
-> converts a monophosphate into a diphosphate.
Nucleoside monophosphate kinases -> converts a monophosphate into a diphosphate.
41
ONE ENZYME converts ALL of the diphosphates into triphosphates: , which is an important enzyme to balance the stoichiometry of triphosphates.
ONE ENZYME converts ALL of the diphosphates into triphosphates: Nucleoside Diphosphokinase, NDPK, which is an important enzyme to balance the stoichiometry of triphosphates.
42
Carbamoyl phosphate synthetase is activated by and
and is inhibited by , , and .
and is inhibited by , , and .
Carbamoyl phosphate synthetase is activated by ATP and
PRPP and is inhibited by UMP, UDP, and UTP.
PRPP and is inhibited by UMP, UDP, and UTP.
43
The second reaction is catalyzed by Aspartate
Transcarbamoylase, ATCase, which has allosteric regulation
and feedback inhibition
. • ATCase is allosterically regulated by 3 effectors:
• (activates), and (activates) • (feedback inhibitor)
Transcarbamoylase, ATCase, which has allosteric regulation
and feedback inhibition
. • ATCase is allosterically regulated by 3 effectors:
• (activates), and (activates) • (feedback inhibitor)
The second reaction is catalyzed by Aspartate
Transcarbamoylase, ATCase, which has allosteric regulation
and feedback inhibition
. • ATCase is allosterically regulated by 3 effectors:
• ATP (activates), and aspartate (activates) • CTP (feedback inhibitor)
Transcarbamoylase, ATCase, which has allosteric regulation
and feedback inhibition
. • ATCase is allosterically regulated by 3 effectors:
• ATP (activates), and aspartate (activates) • CTP (feedback inhibitor)
44
Regulation of the first two enzymes of the pathway is
important for balance:
• a high concentration of
stimulates synthesis of
• high concentration of turns off the
pathway.
important for balance:
• a high concentration of
stimulates synthesis of
• high concentration of turns off the
pathway.
Regulation of the first two enzymes of the pathway is
important for balance:
• a high concentration of purine nucleotides (ATP)
stimulates synthesis of pyrimidines
• high concentration of pyrimidines (CTP) turns off the
pathway.
important for balance:
• a high concentration of purine nucleotides (ATP)
stimulates synthesis of pyrimidines
• high concentration of pyrimidines (CTP) turns off the
pathway.
45
Test Question!
AZT resembles
AZT resembles
Test Question!
AZT resembles thymidine.
AZT resembles thymidine.
46
The azido-group of AZT blocks
• There’s no (mechanism of chain termination)
• There’s no (mechanism of chain termination)
The azido-group of AZT blocks DNA polymerization
• There’s no 3’ –OH (mechanism of chain termination)
• There’s no 3’ –OH (mechanism of chain termination)
47
Viral RNA-dependent DNA polymerase (reverse transcriptase) is
100X more sensitive to than host cell .
100X more sensitive to than host cell .
Viral RNA-dependent DNA polymerase (reverse transcriptase) is
100X more sensitive to AZT than host cell DNA polymerase.
100X more sensitive to AZT than host cell DNA polymerase.
48
Ribonucleotide Reductase (RNR), catalyzes all the conversions from
Ribonucleotide Reductase (RNR), catalyzes all the conversions from NDPs -> dNDPs
49
Ribonucleotide Reductase (RNR): After the is formed (reduced), the enzyme reverses to the state
and is ready for another cycle.
and is ready for another cycle.
Ribonucleotide Reductase (RNR): After the deoxy-sugar is formed (reduced), the enzyme reverses to the oxidized state
and is ready for another cycle.
and is ready for another cycle.
50
RNR regulation: R2 subunit
• The small subunit, R2, forms a that is
needed for the mechanism.
• Cells must control proper balance of ,
otherwise mutations can occur.
• The small subunit, R2, forms a that is
needed for the mechanism.
• Cells must control proper balance of ,
otherwise mutations can occur.
RNR regulation: R2 subunit
• The small subunit, R2, forms a Tyr radical that is
needed for the mechanism.
• Cells must control proper balance of dNDPs,
otherwise mutations can occur.
• The small subunit, R2, forms a Tyr radical that is
needed for the mechanism.
• Cells must control proper balance of dNDPs,
otherwise mutations can occur.
51
RNR regulation: R1 subunit
1) Specificity site: tells the enzyme which to
transform into
2) Activity site: on/off switch. turns the enzyme on. turns the enzyme off (feedback inhibition).
1) Specificity site: tells the enzyme which to
transform into
2) Activity site: on/off switch. turns the enzyme on. turns the enzyme off (feedback inhibition).
RNR regulation: R1 subunit
1) Specificity site: tells the enzyme which NDPs to
transform into dNDPs
2) Activity site: on/off switch. ATP turns the enzyme on. dATP turns the enzyme off (feedback inhibition).
1) Specificity site: tells the enzyme which NDPs to
transform into dNDPs
2) Activity site: on/off switch. ATP turns the enzyme on. dATP turns the enzyme off (feedback inhibition).
52
TEST QUESTION
R1 subunit site -> tells the enzyme which can bind to the active site and transform into .
R1 subunit site -> tells the enzyme which can bind to the active site and transform into .
TEST QUESTION
R1 subunit Specificity site -> tells the enzyme which NDPs can bind to the active site and transform into dNDPs.
R1 subunit Specificity site -> tells the enzyme which NDPs can bind to the active site and transform into dNDPs.
53
dATP and ATP are both purines which favor the binding of (UDP
and CDP).
and CDP).
dATP and ATP are both purines which favor the binding of pyrimidines (UDP
and CDP).
and CDP).
54
dATP inhibits the other ! But it also promotes activity towards
pyrimidines. These are 2 apparently opposite effects and the outcome depends on .
pyrimidines. These are 2 apparently opposite effects and the outcome depends on .
dATP inhibits the other allosteric site! But it also promotes RNR activity towards
pyrimidines. These are 2 apparently opposite effects and the outcome depends on concentration.
pyrimidines. These are 2 apparently opposite effects and the outcome depends on concentration.
55
At very high concentration, dATP inhibits
At moderately high concs, dATP of pyrimidines in order
to balance purines vs. pyrimidines without totally shutting down the enzyme.
At moderately high concs, dATP of pyrimidines in order
to balance purines vs. pyrimidines without totally shutting down the enzyme.
At very high concentration, dATP completely inhibits
At moderately high concs, dATP increases the reduction of pyrimidines in order
to balance purines vs. pyrimidines without totally shutting down the enzyme.
At moderately high concs, dATP increases the reduction of pyrimidines in order
to balance purines vs. pyrimidines without totally shutting down the enzyme.
56
Test Question: Diphosphates bind to the
Test Question: Diphosphates bind to the active site
57
Test Question: Triphosphates bind to the site
Test Question: Triphosphates bind to the specificity site